Jumping Genes: Transposons
Author: Shenzhou
Reviewer: Weiming
Transposons, also known as jumping genes, were first described in 1947 by the renowned American geneticist Barbara McClintock. While studying the unstable inheritance of variegation in the maize aleurone layer, she uncovered a new mechanism by which an intact genetic unit can move from one location in a genome to another. Fu H. and Dooner H. K. examined the phenomenon further in a 2002 paper. Their work showed that, at the molecular level, every organism is a product of continuing genetic recombination: mutations create new sequences, while exchange, insertion, and rearrangement reshape existing ones.
A genetic unit capable of such movement is called a “transposable element,” or transposon. Transposition differs in both concept and mechanism from homologous recombination and site-specific recombination, the latter being a characteristic form of recombination in prokaryotes. The movement of chromosomal fragments through exchange, inversion, translocation, and similar events depends on the RecA, RecB, and RecD recombination proteins. Both the sites and the transferred fragments vary, and ultraviolet radiation or chemical mutagens can increase the frequency of these events. Transposon-mediated recombination, by contrast, depends on a transposase and inverted-repeat (IR) sequences, and mutagens do not promote it. Transposition does not require sequence homology, although transposons do show preferences for certain target sequences. Insertion and reversion mutations can therefore occur at relatively high frequencies. Because a discrete genetic segment moves from one site to another, this independent structural unit is aptly called a “jumping gene.”
In 1947, while investigating the genetic basis of variegated maize aleurone and plant pigmentation, McClintock found that variegation was often accompanied by the characteristic cytogenetic pattern of a chromosome breakage–fusion–bridge cycle.
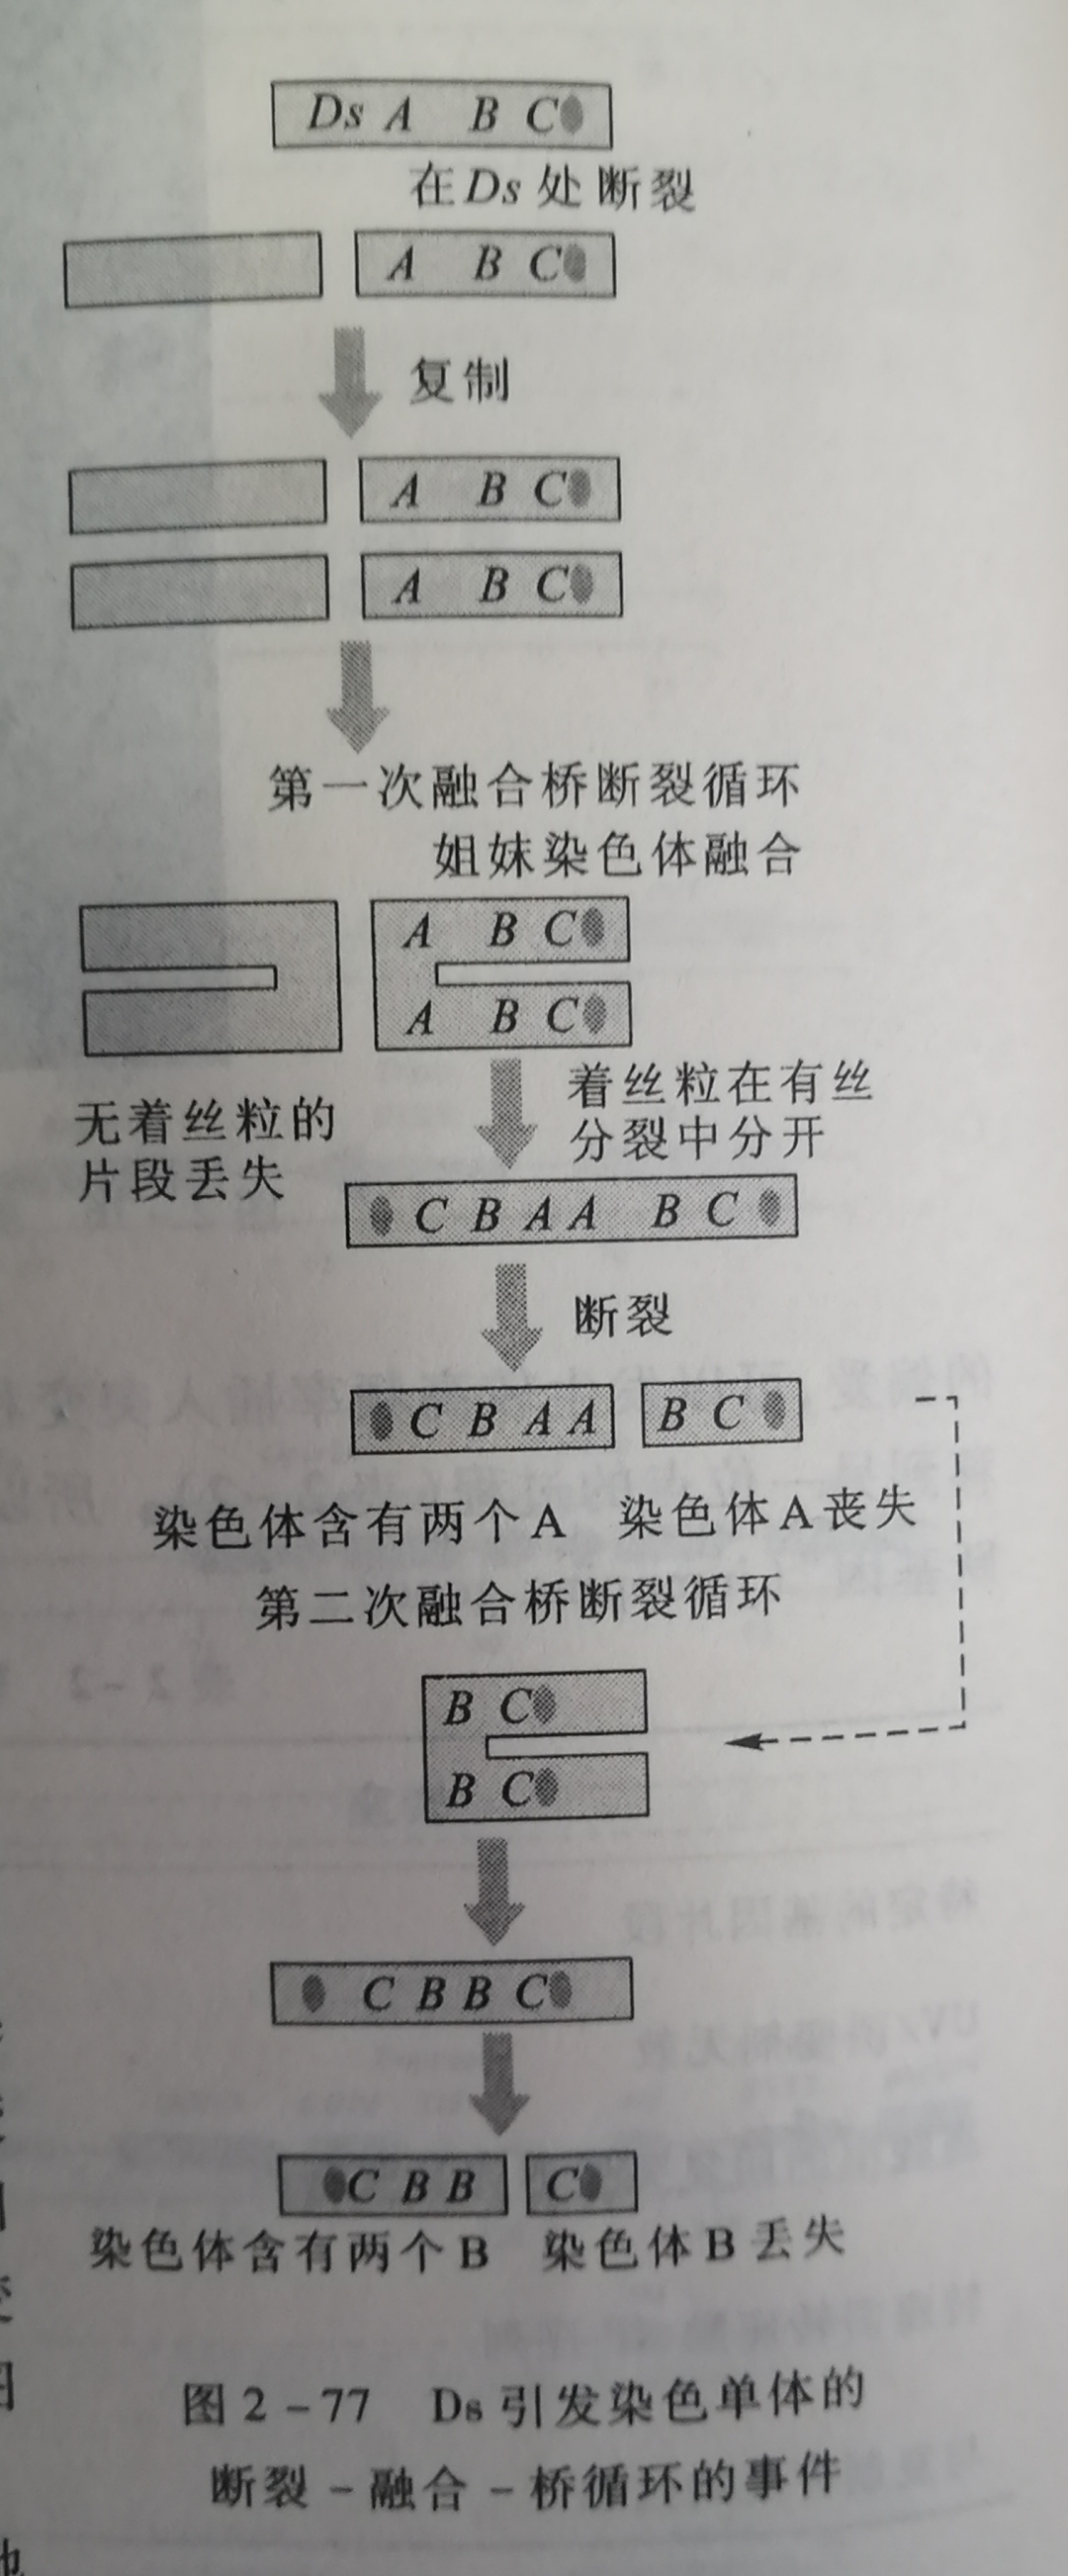
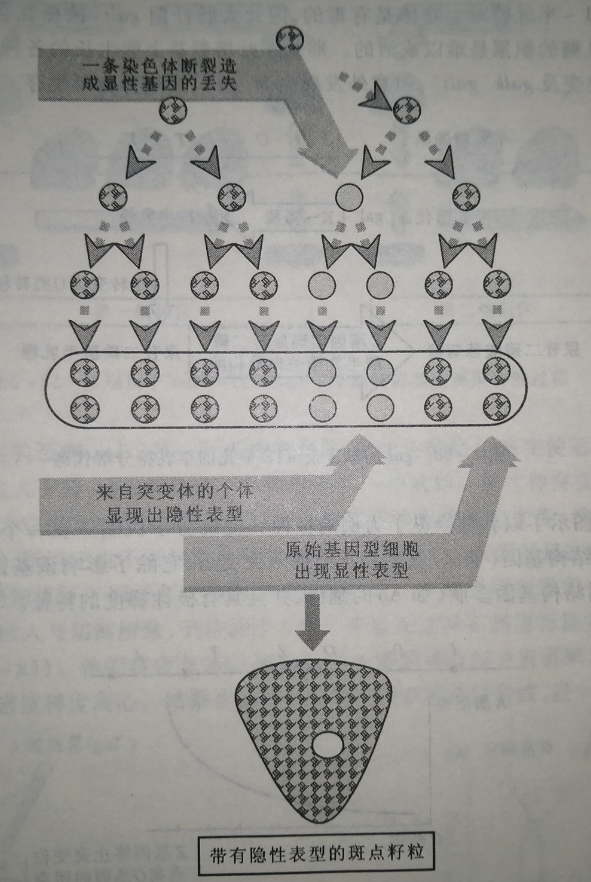
She proposed that chromosome breakage in maize was caused by a Dissociation element called Ds. In a heterozygote, Ds lay between the centromere and certain dominant genes on one homologous chromosome. The other homolog lacked Ds and carried the recessive alleles. A break at Ds produced an acentric fragment that was lost during mitosis, leaving the daughter cells with only the recessive genes on the intact homolog. The centromere-bearing portion of the broken chromosome was left with sticky ends at the Ds break. After replication, those ends fused and produced a chromosome with two centromeres. During the next division, spindle fibers pulled the centromeres toward opposite poles and broke the chromosome again. As the process repeated, it formed a breakage–fusion–bridge cycle.
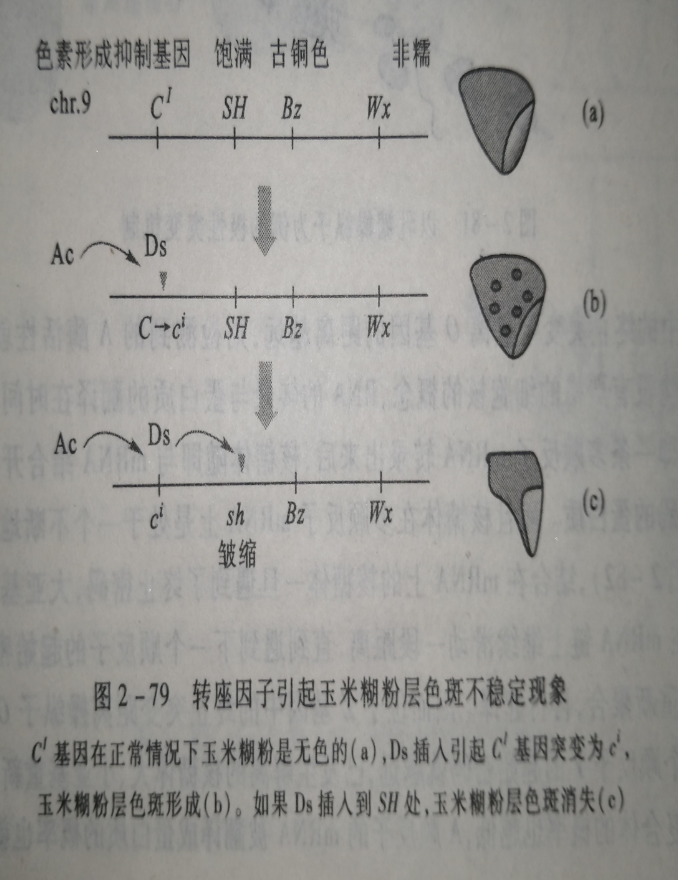
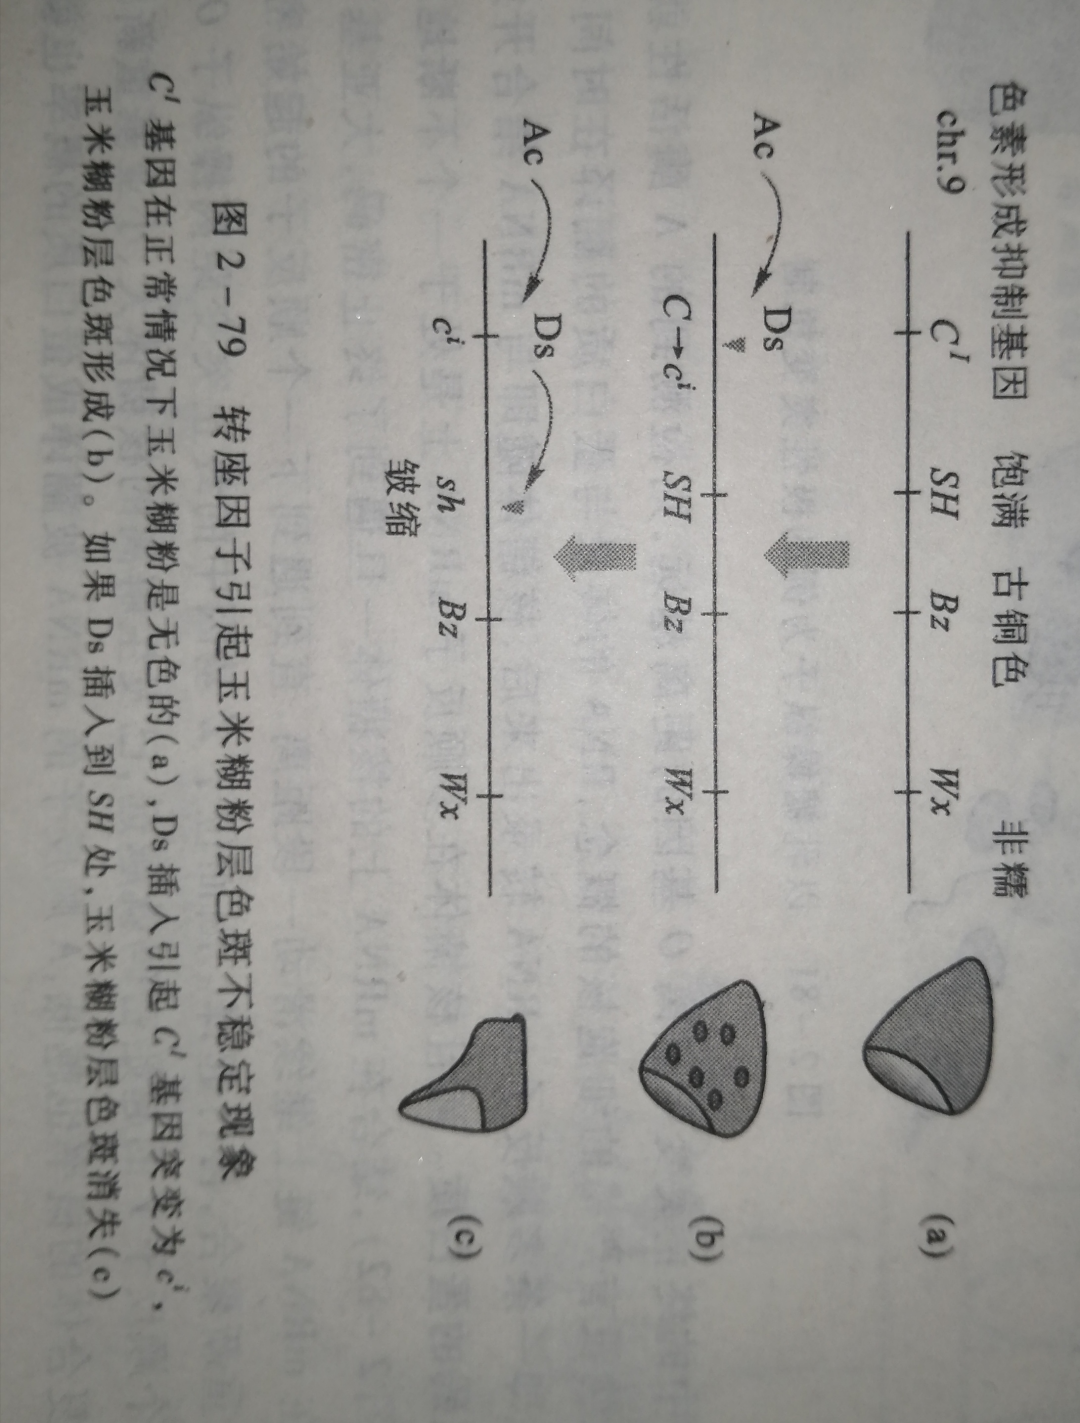
When transposition occurs during the growth and development of a maize kernel, spots appear in its aleurone layer. The earlier the event occurs, the larger the spots; the more often it occurs, the more spots appear. McClintock also showed that Ds is nonautonomous and is controlled by an Activator element called Ac. If Ds inserts into an aleurone pigment gene under Ac’s control and changes it into another allele, variegation appears. A later Ac-regulated jump by Ds can restore the original allele through a reversion mutation, producing the spots’ unstable pattern of inheritance.
 爱发电(点击图片跳转)